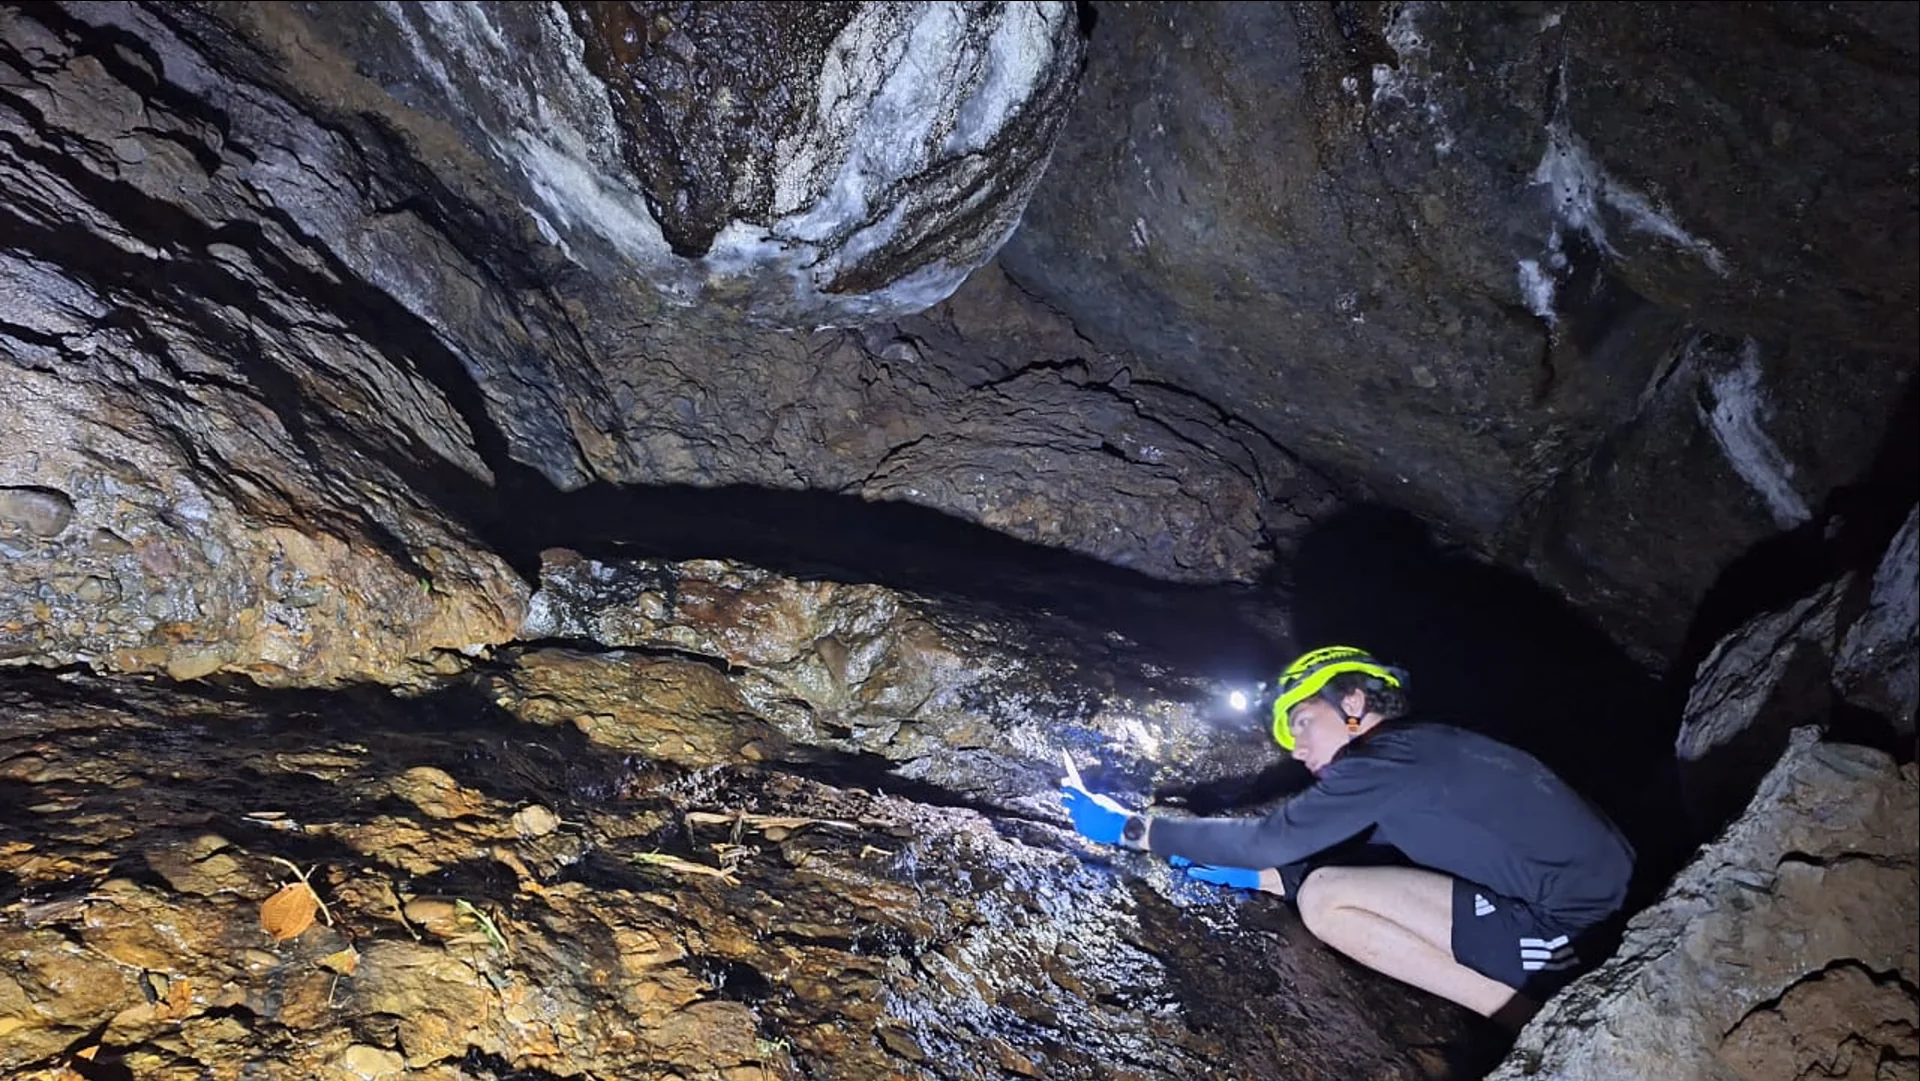
How microbial communities assemble, and whether the state they reach is set by rules or by history.
Sebastian Correa-Gallego
I am a biologist from Jardín, a coffee town on the Western Cordillera of the Colombian Andes. In secondary school I joined OTACA, my school's atmospheric observation group, and reported cloud cover for S'COOL, a NASA program that compared what we saw from the ground with what a satellite recorded overhead. Asking whether two accounts of the same system agree has stayed with me since. At Universidad EAFIT in Medellín, where Dr. Nicolás Pinel advised me throughout my degree, I joined the student research group in microbiology and astrobiology in 2022 and later coordinated it. My thesis followed the cultivable microbial community of the Organal San Antonio, a cave in Támesis, along its gradient of light, often with equipment I had to improvise. A six-month internship in the lab of Dr. Sergio Muñoz-Gómez at Purdue University then took me inside the cell. The lab looks for the physiological principles that constrain how cells evolve, including the role of mitochondria in the origin of eukaryotes. My work there, on how yeasts divide their proteome across carbon regimes, led to a manuscript now in preparation. I am currently applying to graduate programs in ecology and evolution.
As a first-generation student from a rural farming family, I have studied on scholarships at every stage, and Fundación Fraternidad Medellín supported both my degree and my internship at Purdue. I am committed to opening science to students who come from places like mine, where it is not taken for granted.
“It is interesting to contemplate an entangled bank … and to reflect that these elaborately constructed forms, so different from each other, and dependent on each other in so complex a manner, have all been produced by laws acting around us.”
Convergence and contingency recur at several levels of biological organization.
They appear when a community assembles from a pool of species, when an evolving lineage is replayed from the same starting point (Blount et al. 2008), and when cells that once lived apart come to depend on one another (Morris et al. 2012). At each of these levels some outcomes are reproducible and others turn on the order in which things happened. The outcome is probably set neither by rules alone nor by history alone, and what interests me is where the boundary between the two lies and what sets it. More broadly, the questions I would like a career to move through concern the evolutionary transitions in biological complexity (Szathmáry 2015; Ratcliff et al. 2012) and the interactions that make them possible, and microbial cells are the system in which I find them both most tractable and most beautiful.
The cave and the yeast cells looked at first like separate problems. One was a community changing along a gradient of light and the other a cell reorganizing under a constraint imposed on it, and I have come to read them as one phenomenon at two resolutions. Working at both, I would like to bring to fieldwork the same quantitative rigor I learned at the bench. Microbial communities are where the two resolutions meet in a single experiment, because the cells can be characterized before they are combined and the community can be assembled again from the same pool. The sections below follow where these interests lead, first to when communities converge and then to what the physiology of their members might reveal about it.
When is community assembly reproducible, and when does arrival order decide the outcome?
Communities assembled from the same species pool under identical conditions sometimes converge on one reproducible state and sometimes diverge into several, depending on the order in which members arrive (Fukami 2015). Convergence and divergence appear in the same experimental systems. Replicate glucose-limited communities converge at the family level while, for most inocula, their species composition diverges (Goldford et al. 2018), and that divergence can arise from multistability in the population dynamics, with chance deciding which state a replicate reaches (Estrela et al. 2022).
In a model, tradeoffs among growth traits such as lag, growth rate and yield are enough to produce more than one stable state on a single limiting resource (Manhart and Shakhnovich 2018), so the sources of divergence may be partly physiological. Ecology has identified candidate mechanisms for the history-dependent case, such as niche preemption and niche modification, and conditions that favor it, such as a large regional pool (Chase 2003). In the nectar of a hummingbird-pollinated shrub, the bacterium Acinetobacter nectaris arriving first lowers the pH and holds back the yeast Metschnikowia reukaufii. The yeast can evolve resistance, possibly at a marginal cost to its growth, so one environmental factor governs both the ecological and the evolutionary consequences of arrival order (Chappell et al. 2022). Such a factor is identified once a community has formed. What ecology does not yet have is a parameter of the members themselves, measured before assembly begins, that says which regime a given pool will fall into. If such a parameter exists, part of a community's history could be anticipated before it unfolds, which would link cellular physiology to community assembly.
That parameter may lie in how each strain allocates its proteome as its environment changes.
At the level of communities, species traits already predict the strength of priority effects better than phylogenetic relatedness does, once they are separated into niche components such as what a species requires and how it alters its environment, though so far only for pairs of species, and the severity of the nectar environment explained more than any of them (Vannette and Fukami 2014). Microbes in nectar typically acidify it and change its sugars and amino acids, and how far those changes depend on a microbe's genotype and on environmental conditions remains understudied (Quevedo-Caraballo et al. 2025). Both niche components may rest in part on metabolism. In bacteria, a finite proteome is divided between ribosomes, whose share rises with growth rate as nutrients improve, and the enzymes of metabolism (Scott et al. 2010). In this view growth rate is less a trait than a consequence of that division. The same constraint can account for a behavior as specific as overflow metabolism, because in E. coli respiration costs about twice as much protein per unit of energy as fermentation, so fast growth can come at the price of yield and leave by-products in the environment (Basan et al. 2015).
The diversity of niche components among the species in a pool may itself promote historical contingency (Fukami 2015). The hypothesis is that one measurable form of that diversity, the spread of allocation strategies across a pool, predicts how far replicate communities diverge. Within a strain, faster growth can cost yield as conditions change (Basan et al. 2015), but across species growth rate and carrying capacity often rise together (Xiong et al. 2026). In theory, greater variation in growth rates within a pool makes communities develop in a more orderly sequence, from fast- to slow-growing taxa (Deng et al. 2024). The spread that may matter for history is therefore probably not where strains sit on a single axis but how far each one shifts its allocation, and the growth, lag and by-products that follow, as its environment changes, including the changes made by those that arrived before it. A wide spread may strengthen priority effects, if what early arrivals leave behind favors some later arrivals over others, or weaken them, if strains that differ in what they require establish regardless of who arrives first (Debray et al. 2022). Because such responses can evolve while a community assembles, the spread may itself change over time. Assembling pools of narrow and wide spread, matched in how much their members' growth rates vary, under permuted arrival orders, from strains characterized beforehand and ideally isolated from one natural community, such as the microbes of flowers, distinguishes the two. Comparing the predicted regimes with the states that flowers reach in the field would then test the result outside the laboratory. The communities would need to be followed long enough to tell lasting alternative states from transient ones (Fukami 2015), and if spread does not predict divergence in either direction, the hypothesis is wrong.